Mostrando entradas con la etiqueta Plantas. Mostrar todas las entradas

jueves, 2 de abril de 2015

"Las plantas tienen nuestros cinco sentidos y quince más": Stefano Mancuso, neurobiólogo vegetal

Foto: Xavier Gómez
Inteligencia vegetal
Representan el 98,7% de la vida en el planeta; sin embargo, sólo el 3% de los científicos estudian las plantas. ¡Sólo el 3% para estudiar casi la totalidad de la vida! Absurdo. Mancuso es uno de ellos, con más de 250 artículos científicos sobre el tema y que acaba de publicar, con la periodista Alessandra Viola, Sensibilidad e inteligencia en el mundo vegetal (Galaxia Gutenberg), en el que narra los estudios y resultados más recientes, propios y ajenos, y que demuestran que las plantas se comunican entre ellas y con otros animales, duermen, memorizan, aprenden, cuidan de su prole, toman decisiones, e incluso son capaces de manipular a otras especies. Un mundo por descubrir.

Las plantas sienten?
Mucho más de lo que sentimos los animales. Y no es mi opinión o percepción, es una evidencia científica.

No es usted un iluminado.
No. Sabemos que perciben los cambios eléctricos, el campo magnético, el gradiente químico, la presencia de patógenos...

¿Oyen, ven...?
Las plantas tienen nuestros cinco sentidos y quince más. No tienen ojos y oídos como nosotros, pero perciben todas las gradaciones de la luz y las vibraciones sonoras.

¿Y les gusta la música?
Ciertas frecuencias, sobre todo las bajas (entre los 100 Hz y los 500 Hz), favorecen la germinación de las semillas y el crecimiento de las plantas hacia la fuente de ese sonido, que equivale a frecuencias naturales como la del agua que corre, pero hablar o cantar a las plantas es perder el tiempo.

¿Hay sonidos bajo tierra?

Se ha descubierto que las raíces producen sonido y son capaces de percibirlo. Eso sugiere la existencia de una vía de comunicación subterránea.

Tampoco tienen nariz.
Su olfato y gusto son muy sensibles. Perciben las moléculas químicas, es su modo de comunicación, cada olor es un mensaje. Y tienen tacto, basta ver a cámara rápida cómo palpa una planta trepadora.

¿Y dice que se comunican?

Se comunican con otras plantas de la misma especie a través de moléculas químicas volátiles, mandan por ejemplo mensajes de peligro. Si un insecto se le está comiendo las hojas, la planta produce al instante determinadas moléculas que se difunden kilómetros y que avisan de que hay un ataque en curso.

¿Y cómo se defienden?
De muchas maneras. Pueden aumentar sus moléculas venenosas o producir proteínas indigeribles para el insecto. Muchas plantas al ser comidas por un insecto emiten determinadas sustancias para atraer a otros insectos que lo depreden.

Eso es comunicación entre especies.

Las plantas producen muchas moléculas químicas cuyo único objeto es manipular el cerebro de los animales, en ese contexto se inscriben las drogas.

Un ejemplo...
Estudios recientes demuestran que un naranjo o un limonero en flor actúa de diferente manera según la cantidad de polen que lleve el insecto. Si lleva mucho polen, aumenta en el néctar la cantidad de cafeína para activar su cerebro, para que se acuerde de esa planta y vuelva. Si lleva poco polen, corta la cafeína.

¿Inteligencia vegetal?
Si inteligencia es la capacidad para resolver problemas, las plantas son capaces de responder de manera adecuada a estímulos externos e internos, es decir: son conscientes de lo que son y de lo que las rodea.

¡Eso es mucho!

Hemos ignorado cómo funciona el 99,7% de la vida en el planeta y no podemos permitírnoslo porque nuestra dependencia del reino vegetal incluye -además del aire, la comida y los fármacos- la energía (los combustibles fósiles son depósitos orgánicos).

Desconocemos el 90 por ciento de las plantas.

En su evolución las plantas han producido millones de soluciones que son muy distintas de las que han producido los animales. Hasta ahora el hombre ha basado su tecnología en cómo estamos hechos nosotros: un centro de mando y una jerarquía de órganos, y así se organizan nuestras sociedades, gobiernos, máquinas...

Hay otro mundo en el que inspirarnos.
Estudiar las plantas nos dará una cantidad ingente de posibilidades tecnológicas. Por ejemplo, las redes: una red de internet y un conjunto de raíces son muy similares. Pero las plantas son redes vivas, imagine lo que podemos llegar a aprender de ellas.

¿Son altruistas?

Compiten con otras especies y cooperan si son del mismo clan. Pero hay algunos ejemplos extraordinarios en los que podemos hablar de un alto grado de altruismo. Hay una investigación muy hermosa que se hizo hace cuatro años en Canadá.

Cuénteme.
Se aisló a un gran abeto del acceso al agua, y los abetos de alrededor le pasaron sus nutrientes durante años para que no muriera. Las plantas son organismos sociales tan sofisticados y evolucionados como nosotros.

¿Cuidan de su prole?
En las plantas observamos el cuidado parental que observamos en los animales más evolucionados. En un bosque denso, para que un árbol recién nacido adquiera cierta altura para poder hacer la fotosíntesis y ser autosuficiente han de pasar al menos diez o quince años durante los cuales será alimentado y cuidado por su familia.

¿Dónde tienen el cerebro?
Las neuronas son las únicas células en los animales que producen y transmiten señales eléctricas. En las plantas, la mayor parte de las células de su cuerpo lo hacen, y en la punta de las raíces tienen muchísimas. Podríamos decir que toda la planta es cerebro.


ORIGINAL: Vanguardia.es
Victor-M Amela, Ima Sanchís, Lluís Amiguet
31/03/2015

jueves, 27 de marzo de 2014

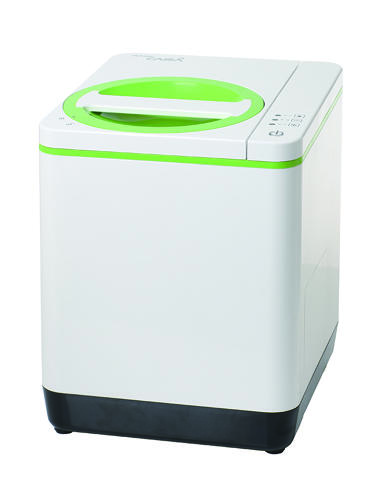
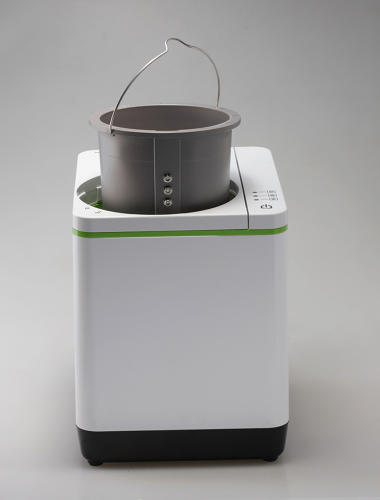
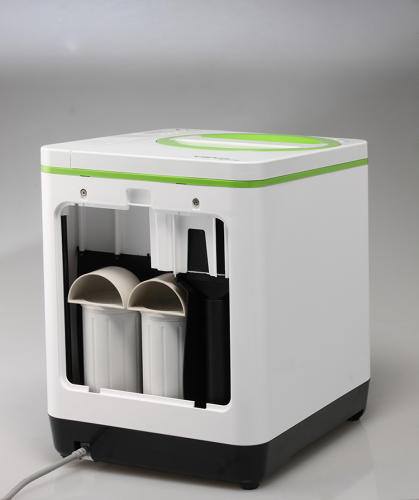
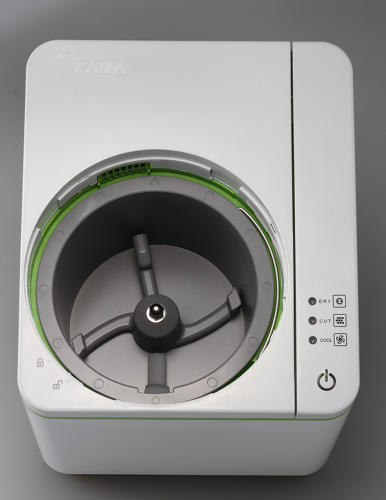
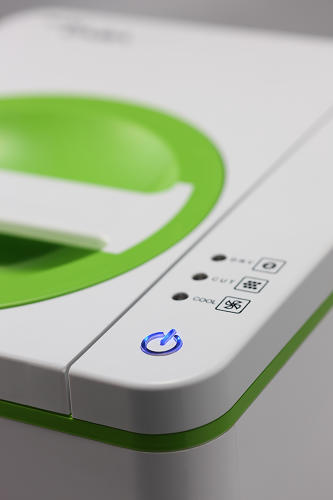
A Countertop Composter That Zaps Your Food Scraps Into Healthy Soil Fertilizer


In just three hours, the Food Cycler turns waste into value--and could hopefully help households cut down on the hundreds of pounds of uneaten food they throw away. 

About 25% of the food in your refrigerator will probably end up in the trash instead of on your plate. And while that’s unfortunate for your wallet, it’s even worse for the environment: The carbon footprint from food waste is actually bigger, amazingly, than the pollution from driving the typical car. Some of the impact comes when the food goes to the landfill, since rotting scraps release the potent greenhouse gas methane.


This is all the reason for a new kitchen device called the Food Cycler Home that aims to make it much easier for people to compost their scraps, even in cities that don't offer composting services (which is most cities). In three hours, it can sterilize and deodorize anything and everything from orange rinds to meat and convert it to a soil amendment that can be safely sprinkled on plants.

The byproduct is organic and looks like coffee grinds. “This will vary slightly depending on what you choose to process, but what is great is that anything you could eat, it could eat--including chicken and fish bones," says Brad Crepeau from the manufacturer Food Cycle Science.

The company, which recently launched a crowdfunding campaign for the Food Cycler on Indiegogo, hopes that the product might offer a viable alternative to the need to create new municipal composting programs. “The challenge with greenbin programs is that they are often costly, and it is sometimes difficult to achieve quotas and sustain widespread buy-in, often because of the odor and unattractiveness of the greenbin and everything that lives in it,” Crepeau says.


A larger version of the Food Cycler has been in use for three years at hospitals, restaurants, universities, and grocery stores, so the company says the technology is proven. But it’s not exactly cheap: The expected retail price is $499, while some chains might offer it for $399.

It also takes a fair amount of electricity as it runs--perhaps not surprising if you’re running something for three hours every day. In a month, it can use about as much as the average dishwasher. It’s not clear how that environmental impact would stack up against something like curbside composting or not composting at all, since that also takes energy, both in driving food away in trucks and running giant commercial composting facilities.

In the end, backyard composting is still probably best for anyone who has the option. Even better is trying to remember to eat the leftovers next time before they turn to mold, so we don't have as much food waste in the first place.

ORIGINAL: FastCo Exist

jueves, 20 de marzo de 2014

ScienceShot: Largest Genome Ever Sequenced

Rob Carr/The Augusta Chronicle/Zuma Press, Inc./Alamy

A loblolly pine tree on the 17th hole of the Augusta National Golf Club in Georgia blocked so many of former President Dwight D. Eisenhower’s shots that in 1956 he tried to get the tree chopped down. Now, loblolly pines (Pinus taeda) are making a different kind of history: Their genome is the largest of any organism yet sequenced. The tree’s extensive use for research and lumber in the southeastern United States made it an early candidate for genetic sequencing. However, its large genome was too cumbersome for conventional whole-genome shotgun sequencing, which sequences short fragments of the genome and then stitches the results together. In a new study, reported today in Genome Biology, researchers bolstered the shotgun approach by preprocessing the individual fragments using genetic cloning, allowing them to more easily assemble the complete genome. Using a single pollinated pine seed, the team assembled the largest genome ever sequenced: 22.18 billion base pairs, more than seven times longer than the human genome. The team found that 82% of the genome was made up of duplicated segments, compared with just 25% in humans. The researchers also identified genes responsible for important traits such as disease resistance, wood formation, and stress response; they did not, however, find any genes for ruining presidential golf games.

See more ScienceShots.

ORIGINAL: Science Magazine
20 March 2014

martes, 18 de marzo de 2014

Bionically Enhanced Chloroplasts Boost Photosynthesis and Spawn a New Field

Photo Credit: Bryce Vickmark Researchers use a near-infrared microscope to read the output of carbon nanotube sensors embedded in an Arabidopsis thaliana plant.

Consider for a moment the magical work done by chloroplasts. These are the plant organelles that absorb light from the sun, convert it into chemical energy and ultimately use it as a building block for synthesizing glucose, the primary source of fuel for both plants and animals. While their achievement has the appearance of alchemy, like every other organelle, these chloroplasts are but little machines. Now, it seems they're due for an upgrade.

In a paper published yesterday in the journal Nature Materials, chemical engineers at the Massachusetts Institute of Technology report that when injected with single-walled carbon nanotubes (SWNTs), chloroplasts can be coaxed to photosynthesize more efficiently than normal.

The first phase of photosynthesis, referred to commonly as the "light reactions," involves excitation of pigments and the subsequent transport of electrons between multiple photosystems. The researchers used this flow of electrons as a measurement for the rate of photosynthesis and found that when the nanotubes were present the flow increased by 49 percent.

Chlorophyll, the pigment normally found in chloroplasts, can only absorb a small fraction of the light entering a plant, most of which resides in the 400 to 500-nanometer and 600 to 700-nanometer range. Although the researchers cannot yet offer an explanation for why carbon nanotubes would enhance the efficiency of chloroplasts, the team theorizes that it may be due to a broadening of this range. SWNTs are known to absorb light in the ultraviolet, visible, and near-infrared spectra.

The MIT engineers write:

"Improving photosynthetic efficiency may require extending the range of solar light absorption, particularly in the near-infrared spectral range, which is able to penetrate deeper into living organisms."

They report having the most success with chloroplasts that had been removed from the plant. Under these circumstances, they were able to inject the nanotubes directly into the organelle. 

In a separate experiment, the researchers sought to find a way to deliver nanotubes into a living plant. In order to do this, they developed a new technique called lipid exchange envelope penetration. Basically, they applied the nanotubes to underside of the leaf via a watery solution which is absorbed through tiny pores called stomata. The transfer across the fatty membrane of the chloroplast was made possible by coating the carbon nanotubes in negatively charged DNA.


When they introduced machinery into a living plant in this way, the chloroplasts received slightly less of a boost, photosynthesizing only 30 percent more efficiently than normal. But this delivery technique may itself be counted as a breakthrough. 

With it, the researchers have tried packing plant cells with particles that protect it from the damaging effects of light exposure, and with another type of carbon nanotube that has been shown to be sensitive to nitric oxide. With such techniques, chemical engineers may one day develop plants that function as pollution detectors. 

Indeed the researchers are arguing that their work establishes an entire new field of research, one they're calling plant nanobionics.

ORIGINAL: IEEE Spectrum
By Morgen Peck
Posted 17 Mar 2014

viernes, 28 de febrero de 2014

PPlanter


PPlanter is a scalable, reconfigurable public urinal and sink that uses modular biofilters to treat urine and wastewater. A network of sensors for automated monitoring and a web/mobile interface enable public feedback and participation in the PPlanter design and propagation of future iterations.

The PPlanter works for both men and women, and conveniently takes up a single parking space so that the entrance is flush with the sidewalk. 

The PPlanter system works as follows:
  • An ADA-compliant sink is supplied with a human powered foot or hand pump connected to a freshwater supply tank. The greywater from the sink, along with soap residue, flushes and cleans the urinal, keeping odor to a minimum.
  • The greywater, soap and urine (blackwater) from the ADA-compliant urinal are funneled to a sealed storage tank. The combined water is then pumped into an adjacent planter that houses bamboo plants set in a lightweight mixture of soil and recycled styrofoam coated in pectin. The water from the urinal and sink is evapotranspired by the bamboo and released into the air as distilled, purified water. The bamboo harnesses the incredible amount of nitrogen and phosphorus found in the urine and uses it to produce more bamboo. With high traffic urinals additional planters can be added to the system.
PPlanter is a finalist in the Urban Prototyping Festival's Open Call, and we are applying for additional funding through Indiegogo.com starting soon (stay tuned!!).

Come to our fundraiser "Refreshed + Relieved" at 111 Minna Gallery on October 8th from 6-9 pm! Then, come see the first PPlanter prototype on October 20th at 5th St and Minna, anytime from 12 - 10 pm!


PPlanter is a rapidly deployable, reconfigurable public urinal and sink that uses modular biofilters to treat urine and wastewater. The network of sensors for automated monitoring and this web site are an integral part for public feedback and participation in the design of future iterations.

Learn more about the project:
ORIGINAL: PPlanter

martes, 11 de febrero de 2014

Plant Talk

Plants communicate and interact with each other, both aboveground and below, in surprisingly subtle and sophisticated ways.

 
© POP_JOP/ISTOCKPHOTO.COM

It’s every plant’s worst nightmare. In the fall of 2009, in a Victorian greenhouse at the Cruickshank Botanic Garden at the University of Aberdeen in Scotland, Zdenka Babikova sprinkled vegetation-devouring aphids on eight broad bean plants and sealed each plant’s leaves and stems inside a clear plastic bag. This was no act of malice, though; it was all in the name of science. 
Babikova, a PhD student at the University of Aberdeen, knew that aphid-infested bean plants release odorous chemicals known as volatile organic compounds (VOCs) into the air to warn their neighbors, which respond by emitting different VOCs that repel aphids and attract aphid-hunting wasps. What she didn’t know was whether the plants were also sounding the alarm beneath the soil surface.

Five weeks earlier, Babikova filled eight 30 cm–diameter pots with soil containing Glomus intraradices, a mycorrhizal fungus that connects the roots of plants with its hyphae, the branching filaments that make up the fungal mycelium. Like a subterranean swap meet, these hyphal networks facilitate the trade of nutrients between fungi and plants. In each pot, Babikova planted five broad bean plants: a “donor” plant surrounded by four “receiver” plants. 
One of the receivers was allowed to form root and mycorrhizal contact with the donor; another formed mycorrhizal contact only, and two more had neither root nor mycorrhizal contact. Once the mycorrhizal networks were well established, Babikova infested the donor plants with aphids and sealed each plant in a separate plastic bag that allowed for the passage of carbon dioxide, water, and water vapor but blocked larger molecules, such as the VOCs used for airborne communication.

Four days later, Babikova placed individual aphids or parasitoid wasps in spherical choice chambers to see how they reacted to the VOC bouquets collected from receiver plants. Sure enough, only plants that had mycorrhizal connections to the infested plant were repellent to aphids and attractive to wasps, an indication that the plants were in fact using their fungal symbionts to send warnings.1

In last 15 years the idea that plants are communicating has become much more accepted. It’s exciting to unravel all these different realms of plant communication.—­Richard Karban, Univer­sity of California, Davis

“When Zdenka first showed us those results it was quite a eureka moment,” says David Johnson, a soil ecologist at Aberdeen who co-led the research. “There was a really striking difference between the insects’ responses to plants with and without hyphal connections. We had more samples to test, but even at that point, it was pretty clear that this is an effective signaling system.”

The remarkable conclusions from this study, published last May, are the latest shoots in a growing thicket of data revealing the unexpectedly complex ways that plants exchange information with one another. Researchers are unearthing evidence that, far from being unresponsive and uncommunicative organisms, plants engage in regular conversation. In addition to warning neighbors of herbivore attacks, they alert each other to threatening pathogens and impending droughts, and even recognize kin, continually adapting to the information they receive from plants growing around them. Moreover, plants can “talk” in several different ways:
  • via airborne chemicals, 
  • soluble compounds exchanged by roots and networks of threadlike fungi, and 
  • perhaps even ultrasonic sounds. 
Plants, it seems, have a social life that scientists are just beginning to understand.

“In the last 15 years the idea that plants are communicating has become much more accepted,” says Richard Karban, an evolutionary ecologist at the University of California, Davis. “The evidence for that is now substantial, and it’s exciting to unravel all these different realms of plant communication.”

Whispers on the wind

 
PLANT CHATTER: Volatile organic compounds (VOCs), first theorized by plant scientists Jack Schultz and Ian Baldwin in the early 1980s, are now a well-known form of plant communication. Maple tree saplings (pictured here) ramp up their own defenses in the presence of herbivore-damaged neighbors.© EERIK/ISTOCKPHOTO.COM

In 1983, plant scientists Jack Schultz and Ian Baldwin reported that intact maple tree saplings ramped up their defense systems when exposed to herbivore-damaged maples. The injured trees, they suggested, were alerting neighbors to the presence of a predator by releasing chemical signals into the air. But the plant research community didn’t buy it. The results were difficult to replicate, critics pointed out, and many questioned how a trait that benefits neighboring plants but not the emitter could be evolutionarily stable. By the late 1980s, “most ecologists felt these ideas had been debunked and that it was time to move on,” says Karban.

A decade later, however, a trickle of more carefully designed experiments began to yield convincing evidence to the contrary. In 2000, Karban showed that wild tobacco plants grown in close proximity to sagebrush plants whose leaves had been clipped became resistant to herbivores, ostensibly in response to VOCs released by the sagebrush.2 Other researchers soon reported similar VOC-induced defense responses—both intra- and interspecies—in several other plants, including lima bean, broad bean, barley, and corn. And in 2006, Karban showed that VOCs released by damaged sagebrush induce herbivore resistance in plants growing at distances of up to 60 cm, well within the range of sagebrush neighbors in nature.3

By now the phenomenon of VOC-based plant communication is well described. In several cases, it has also been demonstrated that volatile cues increase fitness in receiver plants. In one study, lima bean plants exposed to herbivore-induced VOCs lost less leaf mass to herbivores and produced more new leaves than controls, for example.4 But no experiment has yet demonstrated that volatile signaling between neighboring plants can benefit the emitting plant, prompting some researchers to suggest that “eavesdropping” is a more accurate description of what has been observed than “intentional” communication.

Either way, researchers who doubt that plants would have evolved to be altruistic have ruminated on the old question of the evolutionary origins of the phenomenon. Perhaps the ability to synthesize and emit VOCs could simply be an unavoidable consequence of non-communicative functions, such as repelling herbivorous insects and attracting insects that parasitize those herbivores. Another possibility is that external communication channels are merely an extension of within-plant signaling. In sagebrush, lima bean, and poplar, VOCs released from damaged parts of a plant induce resistance in intact sections of the same plant, suggesting that each individual plant uses the signals to coordinate its own physiological responses. “The interplant signaling we see may be a result of plants co-opting that process,” explains Karban.

Alternatively, VOC-based signaling between plants may have been favored because it enhances the “extended fitness” of the emitter by benefitting its related conspecifics: a strategy known as kin selection. This idea gained support from a study published last February, in which Karban and colleagues found that airborne communication was more effective among sagebrush plants that were closely genetically matched than among those that were more distantly related.5 “If communication is more effective among kin, it is less likely that plants are giving away information to potential competitors and more likely that it will benefit close relatives,” says Karban. (See sidebar: “Foliage Family Values.”)

While the evolutionary explanation for volatile communication among plants remains open to debate, researchers have been working to identify and chemically characterize VOCs and to figure out how they encode messages. Gas chromatography–mass spectroscopy has unveiled various compounds that function as plant-to-plant signals, and such work has made it increasingly clear that specific blends of those compounds dictate the content of the messages. In 2011, for example, Japanese researchers found that in herbivore-damaged daisies, eliminating any one compound from a mixture of five VOCs, which induces insecticide production in neighbors, significantly reduced the expression of genes associated with insecticide biosynthesis in those plants.6

“Individual compounds are the words,” says Jarmo Holopainen, an ecologist at the University of Eastern Finland, “and these words are combined to make specific sentences.” Unfortunately, he adds, researchers know little about what these volatile signals mean to a plant and how they are perceived. “We’ve made very little progress in deciphering this chemical code.”
Root rumors

 
THE SECRET SOCIAL LIVES OF PLANTS: Contrary to the long-held idea that plants are uncommunicative, recent research has made it clear that many species conduct lively and informative conversations with one another. Scientists have revealed that plants communicate through the air, by releasing odorous chemicals called volatile organic compounds (VOCs), and through the soil, by secreting soluble chemicals into the rhizosphere and transporting them along thread-like networks formed by soil fungi. And this is more than mere gossip: these signals warn neighbors of the many dangers facing plants.

See full infographic: JPG | PDF© LOGAN PARSONS

Plant gossip is not only spread on the breeze; the rhizosphere crackles with chatter, too. Over the past few years, a team led by Ariel Novoplansky of Ben-Gurion University of the Negev in Israel has produced compelling evidence that plants eavesdrop on hints of their neighbors’ distress through their root systems.

Novoplansky’s team planted six garden pea plants so that each pot contained the roots of two different plants. The researchers then subjected the first plant in each row to drought-like conditions and evaluated the response of its neighbors by measuring the width of the microscopic pores, called stomata, on leaf surfaces, which close in response to drought stress.

Fifteen minutes after drought was initiated, the stressed plant closed its stomata—as did its nearest unstressed neighbor, suggesting some sort of drought warning sign had been passed between the two. After an hour, all five neighbors, each more distant from the stressed plant—the only one that actually experienced drought-like conditions—had also shuttered their stomata, indicating that they, too, received the message to prepare for drought.7 Importantly, in a control setup where root contact between neighboring plants was blocked, pores stayed open, indicating that the message was somehow being passed between roots.

“The finding that plants communicate stress cues via roots was itself novel,” says Novoplansky. “But for me another aspect was more interesting and important: that unstressed neighbors not only responded as if exposed to drought themselves, but also released more of the same cue, which was in turn perceived by further, more remote, unstressed plants.”

Novoplansky’s team has since observed the same phenomenon in garden peas under more realistic, field-like conditions and in three wild plant species, and he suspects that root-based stress cuing could be common in nature.8 The mechanisms underlying this ability are still under investigation, but the cue is almost certainly chemical, says Novoplanksy: when researchers extract soluble chemicals released into the soil by drought-stressed roots and apply them to unstressed plants, they see the same response. His team is currently doing metabolomic studies of root exudates to pinpoint the compound or combination of compounds that carry the message. “The hottest candidate for the vector is abscisic acid (ABA), a hormone involved in plant responses to drought and osmotic stress,” he says. “But I wouldn’t be surprised if it was something else.”

Meanwhile, other researchers are starting to explore another underground plant communication system, one in which messages are sent through the labyrinth of hairlike fungal filaments that festoon the roots of the vast majority of plants on the planet—including important crops such as wheat, rice, maize, and barley. These mycorrhizal fungi are involved in an important mutualistic relationship: in exchange for sugars, they provide plants with much-needed phosphorus and nitrogen. In many cases, the fungi connect the roots of neighboring plants to form common mycelial networks (CMNs), which play a major role in recycling soil nutrients and water. And as Aberdeen’s Johnson revealed last summer, CMNs are also a means of communication. The stringy white hyphae act like fiber-optic cables, carrying information between plants of the same or even of different species. (See “Fighting Microbes with Microbes,” The Scientist, January 2013.)

This idea first gained credence in 2010, when a team at South China Agricultural University in Guangzhou showed that interplant connections via CMNs led to increased disease resistance in healthy tomato plants connected to tomato plants that had previously been infected with the fungal pathogen that causes leaf blight.9 The work of Johnson and Babikova, published last year, provided the first evidence that signals warning of herbivore damage can also be transmitted via CMNs.

“Most research into mycorrhizal networks has focused on their role as biological marketplaces,” says Johnson, “but we’ve now shown that they could have an additional role as a really effective way to transmit messages.”

Subsequent work by Johnson’s group found that CMN-mediated signals elicit behavioral changes within 24 hours of an aphid infestation.10 “That’s important because the signaling has to be quick to be ecologically relevant,” says Johnson.

CMNs may also carry signals over far greater distances than airborne volatiles can. One 2009 study documented a fungal network that wove its way through an entire forest, with each tree connected to dozens of others over distances as great as 20 meters.11 Still, Johnson notes, communication within extensive mycelial networks such as these has yet to be demonstrated in the field.

For Johnson and his colleagues, the next step is to use transcriptomics to see which plant genes are expressed in response to aphid attacks. He says he may also compare proteomic analyses of CMN-connected roots with unconnected roots to identify any compounds that differ between the two systems. But it won’t be easy, he says. “Pinning down the molecules involved is going to be a slog.”

Sounding off

Monica Gagliano’s first attempt to publish evidence suggesting that plants might communicate with each other using sounds was met with rank disbelief. Her manuscript was rejected by six different journals in 2010 and 2011. “It was dismissed as something that is not possible,” says Gagliano, an evolutionary ecologist at the University of Western Australia in Perth.

Undeterred, Gagliano kept plugging away. In April 2012, after she had repeated her experiments and addressed comments from seven different reviewers, PLOS ONE accepted the paper. The study showed that chili plant seedlings grown next to fennel germinated more quickly than seedlings grown with conspecifics. Gagliano and her colleagues suspect the chili plants are compensating for the presence of the fennel, which is known to release chemicals that inhibit the growth of other plants. Remarkably, however, all known inter­plant communication pathways—airborne volatiles, root contact, and common fun­gal networks—were blocked. The results begged for an alternative explanation.

In an article reviewing the evidence suggestive of plants’ use of sound as a communication medium, Gagliano and colleagues cited a study showing that the roots of young corn plants grown in water make clicking sounds, and that when sounds in the same frequency range were played back to the roots, they responded by bending toward the source.13

“We’ve shown that plants can recognize when they’re growing next to a ‘bad neighbor’ and change their growth behavior accordingly, even when we remove all the channels of communication we know about,” says Gagliano. “We also have some evidence that there is an emission [of sound] and a response of some sort. We are not ruling out other possibilities, of course, but we think this other channel of communication might be acoustic.”

Theoretically, she says, sound has several advantages over chemical signaling: it propagates faster and over greater distances, and it can be generated with fewer energy costs.14 But behavioral ecologist Carel ten Cate of the University of Leiden in the Netherlands points out that taking advantage of such putative benefits would require sensory mechanisms yet to be described in plants.15 Plants do generate sounds at frequencies outside the range of human hearing, but it’s not clear how they are produced or whether plants can detect sounds at all. “There are many outstanding questions,” Gagliano admits.

Despite widespread skepticism in the plant research field, Gagliano has received some encouragement. UC Davis’s Karban, for example, is cautiously enthusiastic. “She’s presenting results that don’t fit conventional wisdom . . . but she is repeatedly getting results that are very difficult to explain based on the mechanisms we’re currently aware of,” says Karban, noting the parallels between Gagliano’s struggles and his own situation in the 1990s, when the field was reluctant to entertain the idea that plants can communicate with airborne volatiles. “Whether or not the explanation she favors is the right one,” he adds, “I think that she’s gotten results that, as a field, we need to come to grips with.”

Applications for agriculture?

 
PLANT SENSE: Young chili plants seem to know their neighbors: chilis grown next to fennel germi­nate more quickly than those grown with other chili plants. The question is, how do they do it? Curiously, the effect is still present even when all known inter­plant communication pathways—airborne volatiles, root contact, and common fun­gal networks—are blocked, leading Monica Gagliano of the University of Western Australia to suggest that the plants may somehow be “hearing” acoustic clues.© URSULA ALTER/ISTOCKPHOTO.COM

Whether they’re studying volatiles drifting on the breeze or phytochemicals zipping through subterranean fungi, researchers are now bent on elucidating the relevant receptors and deciphering the molecular lingua franca of plant communication. They could then begin to clarify the ecological significance of the phenomenon and, potentially, help farmers grow hardier crops.

Understanding how plants perceive airborne volatile signals, for instance, could inform the genetic engineering of crops that are hypersensitive to cues from sacrificial “beacon” plants that are deliberately damaged to emit signals that trigger neighboring plants to activate their antipredator and/or antipathogen defenses. And if researchers could pinpoint the compounds that act as vectors for stress cues passed between roots, they could potentially “train” crop seedlings to better cope with drought and other stresses.

“I think it can [be a successful strategy], but we have to put in the work to make it happen,” says Novoplansky. “You’re dealing with farmers’ livelihoods, so you have to be certain it will work in realistic agricultural settings,” agrees Johnson, who collaborates with scientists at the UK’s James Hutton Institute and Rothamsted Research, both of which are dedicated to increasing agricultural productivity. “Applying our limited knowledge [of plant-communication mechanisms] to agriculture is a big jump,” he says, “but it is definitely on the horizon.”

Regardless, one message has emerged loud and clear from those studying this new realm of botanical interaction: despite not possessing eyes, ears, or a nervous system, plants are anything but uncommunicative. Rather, the latest findings speak of a plant kingdom brimming with chatter. “When I did my PhD [in the late 1980s], all this stuff was considered very weird,” recalls Novoplansky. “Today, there is no doubt. We now recognize that plants are capable of some very sophisticated exchanges of information with other plants. This idea is not strange anymore.”
FOLIAGE FAMILY VALUES
In 2007, Susan Dudley of McMaster University in Ontario, Canada, and graduate student Amanda File showed that a beach weed called sea rocket, which is common on the shores of the Great Lakes, senses whether it’s growing among siblings or unrelated plants of the same species. When sea rocket detects strangers, it allocates more resources toward sprouting nutrient-grabbing roots, but when it recognizes kin, it graciously restrains itself.1
Since then, researchers have demonstrated kin recognition in several other plant species. The common model organism Arabidopsis thaliana, for example, reins in root development when growing among brethren. Pale jewelweed (Impatiens pallida), on the other hand, reduces leaf growth and elongates and branches its stems in the presence of kin—likely to reduce shading of siblings in the woody areas where it grows, in which light acquisition is a priority.2
Together with Harsh Bais of the University of Delaware, Dudley has also demonstrated that Arabidoposis’s ability to recognize kin depends on the secretion of soluble chemicals from roots.3 The problem is, the researchers have no idea which compounds are important. “Roots put out a lot of chemicals,” says Dudley, “and we don’t know which matter; which are serving as name tags.”
Nevertheless, researchers have been thinking about the evolutionary dynamics underlying such adaptations. “If plants can recognize their siblings and agree not to waste resources competing against them, then the group as a whole benefits,” Dudley explains. But, she adds, precious few studies have measured whether family groups actually do benefit from kin-dependent behavioral changes. “If we want to test our predictions, we have to see whether differential responses have fitness consequences.”
In 2012, Dudley and File documented some of the first evidence along those lines. They showed that ragweed grown among kin develop larger common mycelial networks—through which plants and fungi trade nutrients—than those grown among non-kin, and that ragweed plants with increased root colonization were better protected against pathogens. Greater fungal abundance was also associated with higher leaf-nitrogen levels, indicative of healthy plants.4 “We have more evidence [that plants benefit from kin recognition] in the pipeline,” says Dudley. “Now we need to see what happens out in the field.”
  1. S.A. Dudley, A.L. File, “Kin recognition in an annual plant,” Biol Lett, 3:435-38, 2007.
  2. G.P. Murphy, S.A. Dudley, “Kin recognition: competition and cooperation in Impatiens (Balsaminaceae),” Am J Bot, 96:1990-96, 2009.
  3. M.L Biedrzycki, “Root exudates mediate kin recognition in plants,” Commun Integr Biol, 3:28-35, 2010.
  4. A.L. File et al., “Plant kin recognition enhances abundance of symbiotic microbial partner,” PLOS ONE, 7:e45648, 2012.

References

  1. Z. Babikova et al., “Underground signals carried through common mycelial networks warn neighbouring plants of aphid attack,” Ecol Lett, 16:835-43, 2013.
  2. R. Karban et al., “Communication between plants: induced resistance in wild tobacco plants following clipping of neighboring sagebrush,” Oecologia, 125:66-71, 2000.
  3. R. Karban et al., “Damage-induced resistance in sagebrush: volatiles are key to intra- and interplant communication,” Oecologia, 87:922-30, 2006.
  4. C. Kost, M. Heil, “Herbivore-induced plant volatiles induce an indirect defense in neighboring plants,” J Ecol, 94:619-28, 2006.
  5. R. Karban et al., “Kin recognition affects plant communication and defence,” Proc R Soc B, 280:20123062, 2013.
  6. Y. Kikuta et al., “Specific regulation of pyrethrin biosynthesis in Chrysanthemum cinerariaefolium by a blend of volatiles emitted from artificially damaged conspecific plants,” Plant Cell Physiol, 52:588-96, 2012.
  7. O. Falik et al., “Rumor has it . . . : relay communication of stress cues in plants,” PLOS ONE, 6:e23625, 2011.
  8. O. Falik et al., “Plant responsiveness to root-root communication of stress cues,” Ann Bot, doi:10.1093/aob/mcs045, 2012.
  9. Y.Y. Song et al., “Interplant communication of tomato plants through underground common mycelial networks,” PLOS ONE, 5:e13324, 2010.
  10. Z. Babikova et al., “How rapid is aphid-induced signal transfer between plants via common mycelial networks?” Commun Integr Biol, 6:e25904, 2013.
  11. K.J. Beiler et al., “Architecture of the wood-wide web: Rhizopogon spp. genets link multiple Douglas-fir cohorts,” New Phytol, 185:543-53, 2010.
  12. M. Gagliano et al., “Out of sight but not out of mind: alternative means of communication in plants,” PLOS ONE, 7:e37382, 2012.
  13. M. Gagliano et al., “Toward understanding plant bioacoustics,” Trends Plant Sci, 17:323-25, 2012.
  14. M. Gagliano, “Green symphonies: a call for studies on acoustic communication in plants,” Behav Ecol, doi:10.1093/beheco/ars206, 2012.
  15. C. ten Cate, “Acoustic communication in plants: Do the woods really sing?” Behav Ecol, doi:10.1093/beheco/ars218, 2012.

ORIGINAL:
The Scientist
By
January 1, 2014 

viernes, 30 de agosto de 2013

The secret inner world of plants

ORIGINAL: ABC Australia

Delve deep inside plants to see the tiny cells from which they are built, captured in stunning detail by scientists from the ARC Centre of Excellence in Plant Energy Biology.
The secret inner world of plants : Plants not only harness the power of our star and use it's energy, they are survivalists. Plants encourage rain, they use physics and chemistry and communicate - they are far more advanced than we once thought.

Quantum coherence: In essence, rather than the energy from a particular photon choosing one route to pass through the photosynthetic system, it travels through multiple channels simultaneously, allowing it to pick the quickest route (See earlier post: http://goo.gl/agp8K )

Capillary action: Sugars produced in leaves diffuse through a network of tube-shaped cells called the phloem. Sugars accelerate as they move, so the bigger the leaves the faster they reach the rest of the plant. But the phloem in stems, branches and the trunk acts as a bottleneck. The major mechanism for long-distance water transport is described by the cohesion-tension theory, whereby the driving force of transport is transpiration, that is, the evaporation of water from the leaf surfaces. Water molecules cohere (stick together), and are pulled up the plant by the tension, or pulling force, exerted by evaporation at the leaf surface. (See earlier post : http://goo.gl/mCmsPL )

Part of the water cycle:
Scientists say the rainforest is critical in generating the streams and rivers that ultimately turn turbines. If trees continue to be felled, the energy produced by one of the world's biggest dams could be cut by a third. The study is published in the Proceedings of the National Academy of Sciences. (See earlier post: http://goo.gl/plP37l )

Plants communicate:
Not just with themselves but with co-dependent species. (See Post Flowers Buzz with electricity : 
http://goo.gl/BUeY8N). Also see information on Grass : http://goo.gl/r0RYtM

Pic Detail:
Plant veins transport water and nutrients to the leaves, where energy from the sun is used to convert carbon dioxide and water into plant sugars and oxygen. The veins then ship the sugars out of the leaf to where they are needed. (Dr Sarah Rich, Plant Biology, UWA)

Main article:
 
http://www.plantcell.org/content/16/7/1650.full

Further reading for the curious: 

This Arabidopsis thaliana (thale cress) plant embryo reveals two leaves and a primary root. Peroxisomes, which break down oils to give the dormant seed the energy boost it needs to become a seedling, have been stained with a green fluorescent dye. Scale: 0.8mm (Simon Law, Whelan Lab)
By using a dye which changes from clear to blue when a particular gene is turned on, this photo reveals which parts of the Arabidopsis thaliana flower are breaking down fat (they're stained blue). Turning fatty molecules into energy is important for flower growth. Scale: 2mm across. (Andrew Wiszniewski, Smith Lab)
It may look like a sea creature, but it's a close up of the female and male parts of a flower (left and right respectively). Pollen grains can be seen in the male anther. The blue areas show the location of genes turned on in response to drought stress. Scale: 0.8mm. (Vindya Uggalla, Whelan Lab)
Flavonoids are pigment molecules that have many roles in plants, including protection from UV rays. By staining this Arabidopsis thaliana embryo, scientists were able to show it could still produce flavonoids, despite a mutation in its DNA. Scale: 0.8mm across. (Andrew Wiszniewski, Smith Lab)
Plant veins transport water and nutrients to the leaves, where energy from the sun is used to convert carbon dioxide and water into plant sugars and oxygen. The veins then ship the sugars out of the leaf to where they are needed. (Dr Sarah Rich, Plant Biology, UWA)
Small root hair cells are sprouting from the primary root of this germinating Arabidopsis thaliana seedling. These hairs provide the root with a greatly increased surface area, aiding in the uptake of water and vital nutrients. Scale: 0.4mm across. (Simon Law, Whelan Lab)
Rather than letting the useful materials go to waste, this plant is pulling them out. The black areas are where this dynamic process is happening. The red blobs are chloroplasts, where sunlight is captured to make energy; the green dots are mitochondria; and the blue areas are cell walls. Scale: 0.291mm across. (Dr Olivier Keech, Smith Lab)
A close up of a poppy flower bud reveals it is covered in tiny hair-like protective structures called trichomes, which provide protection from frost and water loss and can keep predators and pests away. Scale: 30mm across. (Rachel Shingaki-Wells, Millar lab)
The beautiful colours inside this Darwinia leiostyla flower come from pigment molecules called carotenoids. These powerful molecules play an important role in plant development, growth, energy production and cellular protection. Scale: 10mm across (Dr Cathie Colas des Francs, Small Lab)
Arabidopsis thaliana (thale cress) is the lab rat of plant science. Its studied by thousands of scientist around the world because it's easy to grow, highly productive and completes its life cycle in only 6-8 weeks. (Dr Olivier Keech, Smith Lab)
Sugar and proteins are distributed within a plant cell by the actin cytoskeleton - a network of tiny filaments highlighted in this image by fluorescent protein. The oval shaped pores are stomata, which allow carbon dioxide, oxygen and water in and out of the plant. Scale: 0.085mm across. (Dr Olivier Keech, Smith Lab)
When scientists discover a new protein how do they work out what it does? By fusing a green fluorescent protein with the new protein they can track it within the cell - in this case to the endoplasmic reticulum network, a factory that produces and packages proteins and carbohydrates. Scale: 0.072mm. (Botao Zhang, Whelan Lab)

jueves, 1 de agosto de 2013

Plants Grown With LED PAR Light Are Healthier?

ORIGINAL: Exposing The Truth
by Asura 
March 18, 2013

Grow Lights are an amazing addition to indoor growing that may sometimes be expensive and rack up one large electric bill! Though there are many different types of grow lights recommended by long time growers, we’ll go through some scientific research that will initially be controversial to many within industries using them. After learning about Aquaponics our team began to ask questions about what lights are best for growing plants, we were surprised with what we had found.


It turns out that the best type of light for plant growth is the tiny, efficient, cool running Light Emitting Diode! (LED for short) Why and how is this even possible? To answer this question one must learn what plants require to grow, specifically. Plants only feed on very few and very specific light spectrums, the most surprising part of this is that plants DO NOT take in any visible light spectrums whatsoever! Every grow light company which puts their stock into creating a bulb with a “more full visible spectrum than competitors” is utterly useless for growing plants and require far more electricity to power.

Other mistakes most commonly made when using grow lights is that more lumens, UV and heat will bring the outcome of better plants. More lumens, UV rays and heat coming from light sources are all counterproductive to plant growth, this causes plants to burn, dry up, require more water and use far more energy to remain alive rather than using energy for growth. Plant leaves and stalks do not need to be beamed upon with intense heat energy and radiation, more importantly it is the roots that must remain at a special temperature. During hours of light leaves collect radiation from spectrums that are invisible to the human eye while during hours of darkness they open stomata, best comparable to pores in human skin, to breathe, take note that only the roots of plants drink water and send it through the stems similar to a highway.


As illustrated in the pictures above and below, the two types of chlorophyll will ONLY absorb certain light spectrums known as Photosynthetically Active Radiation (PAR). Having a more full spectrum for plant growth is completely unnecessary, one chlorophyll type absorbs red light between the 630nm and 760nm light spectrum while the other absorbs blue light between 280nm and 460nm. The use of LED lights solves the problem of electricity being wasted on light spectrums that plants can not take in by allowing for each LED to beam very specific ranges of light. Many have recommended using 
  • 2/5ths of a red spectrum,  
  • 2/5ths of a blue spectrum and 
  • 1/5th UV spectrum 
to keep accepted light spectrums well balanced. Each type of plant may require more blue types or red types of light spectrum, it never hurts to perform more research on each specific plant’s requirements.


LED lights run at cool temperatures and don’t create anywhere near enough heat to be significant to plants or animals, yet for plant care it turns out that heat should be highly regulated and does not have to come from lights. As long as the temperature in a room is regulated then no heat is needed from lighting.

The Effects of Temperature On Plant Growth


The efficiency of LED lights in both specific spectrum abilities and low electricity requirements are certainly proving to be an innovative and sustainable solution to plant growth. The Growblu website contains a lot of informational PDFs to quickly and easily justify using LED lights rather than outdated bulb types.

How Light Spectrums Affect Plants

Pretty large forum of invaluable information
ICMag

viernes, 26 de julio de 2013

The Mechanism Determining Plant Height and Leaf and Seed Size - Balance between three proteins controls plant-cell elongation -

ORIGINAL: AIST

- Balance between three proteins controls plant-cell elongation -
(Translation of AIST press release on November 19, 2012) Points
Identification of three types of protein controlling plant-cell elongation
Elucidation of a new mechanism by which each of the three types of protein antagonistically affects the activity of others
Expectations of the development of new crops and garden plants with modified plant height, leaf and seed size, and morphology Summary

Masaru Ohme-Takagi (Invited Senior Researcher), Miho Ikeda (Collaborative Researcher, Restart Postdoctoral Fellow of Japan Society for the Promotion of Science), and co-workers of Plant Gene Regulation Research Group, the Bioproduction Research Institute (Director: Yoichi Kamagata) of the National Institute of Advanced Industrial Science and Technology (AIST; President: Tamotsu Nomakuchi), have confirmed that the length of a plant cell is controlled by the antagonistic actions of three types of protein.

Cell length directly affects plant height and leaf and seed size. The researchers have identified two proteins, PRE1 and ACE, which act as a positive regulator for cell elongation, and one protein, AtIBH1, which inhibits cell elongation. They have found that ACE directly induces cell elongation, whereas AtIBH1 inhibits the activity of ACE by interacting with it. PRE1 indirectly promotes elongation by interfering the activity of AtIBH1. Final cell length is determined by the balance between the three proteins.

These proteins are transcription factors controlling functions of several genes. Use of these transcription factors would make it possible to modify plant height, leaf and seed size, flower and plant morphology, etc. They are expected to be applicable to a variety of areas, including improvement in the efficiency of farming, creation of large plants suitable for biofuel production, and development of unique garden plants.

Details of the results will be published in a US scientific journal, The Plant Cell.
Effect of differences in cell length on plants (Arabidopsis thaliana).

Social Background of Research

Plants, which are important resources, have been traditionally used as food, clothing, and home-building materials, and have comforted people as garden plants. Recently plant-based pharmaceuticals, biofuels, and industrial materials become popular and their application has been increasing. Modifying plant morphology and size to suit different applications should increase the efficiency of production.

From this perspective, modification of plant-cell length is an important subject of breeding studies because it directly affects tree and plant height and leaf and seed size. There are various environmental factors that determine cell length, including sun exposure, temperature, water contents, and nutrient ratios. It is not known how a plant determines its cell length in response to these environmental conditions.

History of Research

AIST has been studying plant genes, particularly the transcription factors that control the actions of many genes, in order to apply them to the production of industrial materials, medicines, and food. The Chimeric REpressor Gene Silencing Technology (CRES-T) and the transcription factor library developed in these studies are being used worldwide as general-purpose tools for a variety of basic and applied transcription factor studies. In addition to the development of such general-purpose tools, AIST is also studying functions of individual transcription factors involved in various phenomena, such as plant morphology, size, and substance production. In the present study, the researchers investigated the mechanism by which plant-cell elongation is controlled.

This study was supported by a grant-in-aid for JSPS Fellows, titled “Isolation of Transcription Factors Controlling Branching, Dwarfing, and Differentiation Potency Applicable to General Crops and their Use (FY2011–2013).”

Details of Research

Plants control cell elongation in response to various environmental conditions, such as sun exposure, temperature, water, and nutrient ratios, and to grow into forms adapted to their environment (e.g. a sunny or a shady location). When, and which, cells are to be elongated is related to seasonal differences in growth (e.g. the elongation of shoots in spring) and to changes in growth over time (e.g. young plants grow vigorously, whereas old plants grow very little). In addition, plant-cell elongation is involved not only in simple growth but also in important plant functions, such as the blooming of a flower and the turning of a flower toward the light when a plant falls over (Fig. 1).

Figure 1 : Examples of phenomena in which plant cell elongation is involved

The researchers have identified three transcription factors from a model plant, Arabidopsis thaliana: PRE1 and ACE, which enhance cell elongation, and AtIBH1, which inhibits cell elongation. These three transcription factors control plant size by regulating cell elongation, without affecting the number of cells. ACE activates the expression of enzyme genes that promote cell elongation. AtIBH1 inhibits cell elongation by interacting with ACE and interfering with its function. PRE1 interacts with AtIBH1 and thus interferes with its inhibition of ACE, thus promoting cell elongation. The researchers named the mechanism of this antagonistic inhibition by ACE, AtIBH1, and PRE1 a tri-antagonistic bHLH system (Fig. 2). Similar mechanisms of antagonistic inhibition, but between only two factors, have been reported in human beings, but mechanisms of antagonistic inhibition by three factors have not been reported before in plants or animals. The tri-antagonistic system is thus a new control mechanism.

Of the three types of transcription factor that were discovered, PRE1 was abundant in stem tips and young leaves and seeds, whereas AtIBH1 was abundant in hardened stem bases, old leaves, and mature seeds. This suggests that the antagonistic inhibition by the three factors, ACE, AtIBH1, and PRE1, regulates the elongation of various cells in each growth stage of the plant.
Figure 2 : Tri-antagonistic bHLH system controlling plant-cell elongation

Future Plans
The researchers aim to develop a technology for modifying plant height and leaf, flower, and seed size by partially enhancing or inhibiting with the functions of PRE1, AtIBH1, and ACE. They will then apply the technology to crop breeding. It is expect that manipulation of these three factors will change plant morphology, as well as its metabolism. They intend to conduct research in the effect of these factors on the metabolic system of plants.